Showing posts with label plant. Show all posts

Thursday, January 11, 2018

The Seeds of Inheritance

Biology Concepts – pollen, plastid inheritance, gymnosperms, angiosperms

I am coming to believe that plants are more complex than animals, even more complex than females. Female plants must be the most difficult things on Earth to understand!

Complete flowers have both anthers for pollen and pistils for egg 
fertilization. Incomplete flowers occur on dioecious plants, 
and have either the pistil (gynoecious) or the anther 
(androecious). Dioecious plants cannot self pollinate, unless 
they have both types of incomplete flowers, like coast
redwoods (see last picture).
Yes, there are female plants. In the plant world, species can be monoecious (mono = one, and ecious = household) or dioecious (di = two). Monoecious plants have individuals that produce both male microgametophytes (pollen) and female megagametophytes (oocyctes or ovules). The individual dioecious plants are either androecious (pollen producing) or gynoecious (seed producing). It's okay to ask if a plant is female, but you still shouldn’t ask her age.

This isn’t even the tip of the tip of the iceberg when it comes to diversity in plant reproduction. There are also different ways to produce seeds. The gymnosperms have unenclosed seeds (gymno = naked, and sperm = seed). Gymnosperms include the conifers (cone producers), the cycads that we talked a little about a few weeks ago, and the gnetum plants. Gnetum plants live close to the equator around the globe and include the Ephedra species. It is from these plants that we get ephedrine and pseudoephedrine that work to relieve allergy and cold congestion.

The other type of seed plants is the angiosperms (angio = hidden). These are the flowering plants that have seeds encased in fruits or other structures that help to protect them and to encourage their dispersal.

One way that the gymnosperms and angiosperms differ is in how they inherit their plastid organelles. But even here there is a lot of overlap and exceptions; plants just keep getting more complex.

Gymnosperms have there seeds exposed on the scales
of the cones, while angiosperms have the protected
inside the fruit (except for strawberries).
Angiosperms have a maternal inheritance of chloroplast DNA (cpDNA), much like animals have maternal inheritance of mitochondrial DNA (mtDNA). The reasons for maternal inheritance of cpDNA elude me. For mitochondria, the theory is that damage to the sperm mitochondria would occur during the swim to the oocyte, so it would be smart to ban them from the egg.

But cpDNA is much more passive, they do not have to do a huge amount of work to get to the ovule of the pollinated plant. The pollen tube grows down to the ovule and delivers the sperm cells right to the egg. There must be some other reason, but I don’t know what it might be.

However, there seem to be more exceptions in angiosperm inheritance of cpDNA than there is in animal mtDNA. A few families of plants, like alfalfa (Medicago sativa) and kiwi fruit vine (Actinidia deliciosa), have a strict paternal inheritance of cpDNA.  This is odd since, the angiosperms have a couple of mechanisms for keeping the plastids out of the male gametes.

Every plant species has a distinct pollen shape, which
is why you can be allergic to some plants and not
others. But each pollen grain has the vegetative cell
that becomes the sperms cells and the tube cell. The
tube usually grows from the side that rests on the
fertilized stigma.
The pollen grain contains a few different kinds of cells. There are one or more generative cells; these are the reproductive cells of the pollen. There will also be many non-vegetative cells as well. The generative cell has two nuclei. One will divide to become the two sperm cells, while the other will form the tube cell to deliver the  sperms cells to the ovule.

In many species, when the generative nucleus divides to form sperm, the plastids are partitioned off, and are not included in the sperm cells. This works to ensure maternal inheritance. In other species, the sperm cells may include plastids, but these quickly degenerate and are not delivered to the ovule. Somehow, the alfalfa plants have overcome these mechanisms and even invented a new one to eliminate or exclude the plastids from the ovule, giving strict paternal inheritance.

Going beyond the alfalfa and kiwi fruit ability to preserve their paternal plastids is the fact that a full 20% of angiosperms can show (but don’t have to show), bipaternal inheritance of cpDNA. This is called potential bipaternal plastid inheritance (PBPI) and is controlled by a male gametic trait, called of all things - PBPI trait! Therefore, the fairly strict maternal inheritance of mtDNA in animals (blue mussels excepted) is not matched by cpDNA in angiosperms.

But it gets weirder. The angiosperm exception is normal for the gymnosperm. Gymnosperms tend to have paternal inheritance patterns for cpDNA. This difference is important to note, since scientists often try to use cpDNA inheritance patterns to track seed movements around the world and through evolutionary time, just like human populations are often tracked using mitochondrial ancestry and inheritance.

But this must be frustrating, because there are also exceptions in the paternal inheritance pattern in gymosperms. The Chinese fir (Cunninghamia lanceolata), which isn’t a fir, is native to Asia but was brought to America in the 1800’s. Remember that before molecular biology, most taxonomic classifications were made on just the morphology (shape and look) of an organism, and its grouping and name were based on how it compared to other organisms. Names often get stuck in the language and are hard to change, so many of the misnomers persist.

Godzilla, or Gojira, always seemed surprised when
the other monster grabbed his tail. Here it happens
to be a giant wolfman. Everybody cashed in on the
werewolf brand; I am surprised Abbott and Costello
aren’t in that picture somewhere.
Consider this, we now know that the Japanese pronunciation for the big green movie monster is “go-zeer-a” or “go-jeer-a,” as it was a portmanteau of the Japanese words for gorilla and whale. But when it came to America, it was just assumed that the name was mispronounced in English and that it was supposed to be “god-zill-a.” We know it is wrong, but the wrong name still survives; it's what you get used to that sticks around.

But back to the Chinese fir. This gymnosperm is a conifer that can grown 150 feet tall, but flaunts its individuality by having a maternal inheritance pattern for cpDNA – much more angiosperm-like behavior than gymnosperm. And this is even odder because the Chinese fir is an older gymnosperm, a much more distant relative to the angiosperms than many gymnosperms that have a strict paternal cpDNA inheritance.

Gymnosperms that show maternal cpDNA inheritance are rare, or just less studied, so one might assume that paternal cpDNA inheritance is fairly strict – wrong. Many gymnosperms have bipaternal inheritance patterns of plastids, so the mechanism might be different from angiosperms, but is no more consistent than that of the flowering plants.

Finally, there is the issue of crossbreeding. In this animal mtDNA and plant cpDNA seem to be similar. Whatever the dominant form of inheritance is seen in natural breedings, the numbers get screwed up when cross breeding occurs. We saw that paternal inheritance of mtDNA in mice was much likely in the mating of different species (interspecific breeding).

The passionflower vine can grow to be 10 meters high
and is the source of the passion fruit that I enjoy so
much. The fruit protects the fertilized seeds that
probably have paternal cpDNA, since most of the
varieties we eat are hybrids of different species.
In plants, this also holds, and may even be more discrepant. Take the passion flowers  (family Passiflora) for instance. Intraspecific breeding (same species) showed the maternal cpDNA inheritance one might expect. But in interspecific crosses the inheritance was 100% paternal. This must represent some attempt to limit the genetic diversity of the organellar genomes, but I leave it to you to explain the reason for it.

The similarity between mitochondrial and plastid inheritance in hybrids brings up another issue – what about mitochondrial inheritance patterns in plants?

It turns out that most plants that have been studied for mtDNA inheritance have a maternal inheritance pattern, just like animals. Amazingly, this includes the gymnosperms, most of which have paternal inheritance of cpDNA. But even some plants with maternal cpDNA patterns can pass on paternal mitochondria. An example of this is the banana - tomorrow morning you can feel like a rebel for garnishing your cornflakes with such an outlaw fruit.

However, the reason would be different. Remember that sperm have their mitochondria in their tails, and in most animals, this is not included in what enters the egg or is degraded just after entering. But few plants have flagellar sperm (like the cycads we talked about before). The sperm mtDNA is not exposed to anymore oxygen radical damage than the ovule mtDNA, yet there is most often uniparental, maternal inheritance.

Coastal redwoods can reach up to 110 meters
(360 ft) tall, but their roots may only go 6 ft.
underground. What's holding this tree in place?
It has two different types of leaves, and has male
and female branches and flowers, but all its
mitochondria and chloroplasts come from one
place, its father.
The interesting cases are those like the gymnosperms; paternal cpDNA, but maternal mtDNA. Once again, the plants are much more complex and intricate in their behaviors than animals, as two separate mechanisms for organellar retention and degradation must be at work in these plants. But even here there can be exceptions. The coast redwood (Sequoia sempervirens) has normal gymnosperm (paternal) inheritance of cpDNA, but it also has paternal inheritance of mtDNA! And the Chinese fir, which breaks the rules and is a gymnosperm with maternal inheritance of cpDNA, also makes itself exceptional in that it has paternal inheritance of mtDNA! Very confusing.

So mitochondria and chloroplasts both work in energy production, both evolved through endosymbiosis, both have single, circular chromosomes (with exceptions), and both have uniparental inheritance patterns (with exceptions). Next week, let’s look a behavior that is different in these two organelles.


Zhang Q, & Sodmergen (2010). Why does biparental plastid inheritance revive in angiosperms? Journal of plant research, 123 (2), 201-6 PMID: 20052516

Bendich AJ (2013). DNA abandonment and the mechanisms of uniparental inheritance of mitochondria and chloroplasts. Chromosome research : an international journal on the molecular, supramolecular and evolutionary aspects of chromosome biology, 21 (3), 287-96 PMID: 23681660


For more information or classroom activities on monoecious/dioecious plants, angiosperms, gymnosperms, or plastid inheritance, see:

Monoecious/dioecious –

Angiosperms –

Gymnosperms –

Plastid inheritance -

Thursday, December 28, 2017

When Is A Chloroplast Not A Chloroplast?

Biology concepts – gravitropism, plastid, chloroplast, chromoplast, amyloplast, leucoplast, malaria parasite

Believe it or not, the way plant roots know to grow into the dirt is related to photosynthesis! “How can this be?” you ask. Well, let’s talk about it.

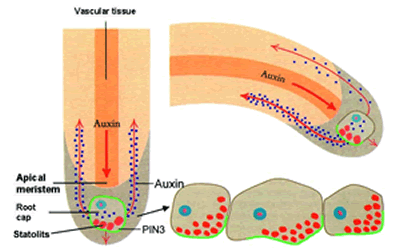
The cells in the tips of the plant rootlet respond positively to gravity, called gravitropism (the older word for it is geotropism). If you lay a growing plant on its side, the roots will respond by growing (turning) toward the gravity within 10 minutes. The mechanism for this stimulation involves tension and a plant hormone called auxin.

Auxin is a growth hormone that gets redirected
in the growing plant root. The statoliths settle
and trigger the hormone to some cells more than
others. Auxin means ”to grow” in Greek, but in
some cases, like in gravitropism of roots, it
actually inhibits growth.
The root cap (the cells at the tip of the root) have some specialized cells called statocyte (stat = position, and cyte = cell). Inside the statocytes are dense granules called statoliths (lith = stone). The statoliths are made of densely packed starch and are a specialized type of organelle called an amyloplast, which is used in many plant cells for storing carbohydrate in the form of starch (amylo = starch). The statoliths are denser than the cytoplasm of the cell; they don’t just float around, they settle out according to gravity.

Since the statoliths are connected to the membrane of the cell by the cytoskeletal actin molecules, so when they settle toward gravity, some cells in the membrane are stretched and some are compressed. This tension signals the cells to change the number of receptors for the growth control hormone auxin. More tension (more stretch) causes the auxin to move away, toward cells that are under less tension. Auxin prevents cell enlargement and cell division, so those root tip cells on the bottom receive more inhibition. Those on top enlarge more and divide more, so the root turns down. If the root is already vertical, the tension is equal in all directions, and the growth is equal in all directions – the root gets thicker and longer.

Gravitropism is related to photosynthesis in that both mechanisms involve chloroplasts, sort of. Root cells don’t perform photosynthesis, they are underground, so they don’t have chloroplasts. But they do have the amyloplastid statoliths, and these are related to chloroplasts.

Both amyloplasts and chloroplasts are specialized versions of the plant organelle called the plastid. We asked last week about what defines a plant cell – maybe the plastid is it. All plant cells have some plastids, but in different plant cells they may take different forms, including chloroplasts, chromoplasts, leucoplasts, amyloplasts, elaioplasts, or proteinoplasts, but they all start out as proplastids (pro = early and plastos = form in Greek).

Proplastids are in every new plant cell. From there
they can differentiate into other forms, including
the chloroplast. Other plastids are used for storage
or biochemical production. We will talk about statoliths
again when we discuss proprioception.
When a cell divides, each daughter gets its share of proplastids, and then depending on the chemical signals that the daughter cell receives, the proplastid will differentiate (from latin, means to make separate) into the types of plastids that the cell needs. A proplastid can become any type of plastid, and from time to time can change between forms as the plant cell requires. Think of it as a sort of stem cell inside a plant cell – if the cell happens to be in the stem of the plant, it could be a stem cell inside a stem cell!

Proplastids become etioplasts, chloroplasts or leucoplasts. The etioplast is a sort of pre-chloroplast; a chloroplast without chlorophyll. It is waiting to be stimulated by light energy before it decides to spend all the energy it requires to make the chlorophyll. The old science fair project about growing bean plants in the dark demonstrates the etioplasts. The plants are white when grown in the dark, but bring them into the light and they soon green up. The sunlight stimulates the etioplasts to make chlorophyll, become full-fledged chloroplasts and start photosynthesizing.

This is a photomicrograph of the plastids of a
red flower petal. The chromoplasts hold the
xanthocyanin pigments, but we see it as a
continuous color because they are so small.

If the proplastid does not differentiate toward a chloroplast pathway (etioplast too) then it will become a leucoplast (leuko = white). The leucoplasts don’t have color; they become specialized for the storage of plant materials. If they store starch, they are called amyloplasts. Lipid storing leucoplasts are called elaioplasts, while protein storing plastids are called proteinoplasts. Each type serves a crucial purpose in the cells they inhabit, and they can all interchange, depending on the conditions the plant cell finds itself in.

Even more important, leucoplasts that are not serving as storage organelles have biosynthetic functions. They work in the production of fatty acids and amino acids. Amino acids link together to from proteins, so their synthesis is very important for plants. Plants must manufacture every amino acid it needs, whereas we get many of ours in our diet. There are even some amino acids that humans can’t make, called the essential amino acids. Of the twenty common amino acids, nine of them must be taken in through our diet, and some people with pathologies can’t make up to seven more. Plants don’t have this luxury; all their amino acids must be made on site. Good thing they have leucoplasts.

There is one other type of plastid that we haven’t talked about, the one that is important for the Autumn tourist trade. Etioplasts and chloroplasts can differentiate into chromoplasts, organelles that store pigments (colored molecules) other than chlorophyll. Chlorophyll provides energy through photosynthesis, but they also have a cost. The old saying, “It takes money to make money” applies to plants as well. It takes energy to make chlorophyll, so it only pays to make chlorophyll when there is ample sunlight to put through photosynthesis. When the days get shorter, the profit margin for producing chlorophyll goes down, so the plant just stops making it.

Twin females were imaged after a lifetime of smoking or non-smoking.   
Can you guess who was exposed to the oxygen radicals in cigarette
smoke her whole adult life?
The oxygen produced in plant cells during photosynthesis can damage many molecules; oxygen likes to react with other compounds and steal or donate electrons. This oxidative damage can wreak havoc with the cells, just look at the face of a long time smoker – the damage and aging process from the oxidants in cigarette smoke will be evident. The chromoplast pigments, like carotenoids (oranges and yellows) and xanthocyanins (reds and purples), can serve as antioxidants, and protect the other cell structures from the damaging effects of oxygen.

So the chloroplasts lose their chlorophyll in autumn and could be called leucoplasts, but the chromoplasts still have the pigments that had been masked by the greater number of chlorophyll molecules. The trees turn magnificent colors and bring people from the cities to stay in bed and breakfasts, and to purchase handmade scarves and way too much maple syrup and apple butter. Economy and biology are so often interrelated.

Plastids are the quintescential plant organelles – no plant cell is without them in some form (well O.K., there is one exception, we’ll talk about that next week). But that still doesn’t mean that they define a plant cell. Remember that algae are not plants, but they have chloroplasts, and chloroplasts are one type of plastid. There is even a bigger exception in this area; some of the apicomplexans.

Certain protozoal organisms, including the malaria parasite (Plasmodium falciparum) contain an organelle called an apicoplast. P. facliparum or its ancestor obtained an algae cell by secondary endosymbiosis (the primary endosymbiotic event was the algae taking in a cyanobacterium), so the apicoplast has a four, not two, membrane system.

The apicoplast of the malaria parasite is of plastid
origin, but it undergoes some unplant-like changes
during cell division. Image D with the branched
apicoplast is my favorite. Those in panel F will
grow to look the one in panel A.
The apicoplast does not perform photosynthesis; we aren’t exactly sure what it does – but it is crucial for the survival of the parasite. It is located in the front of the parasite (in the direction it moves and invades cells) and is always close to the nucleus and the mitochondrion. This suggests some role(s) in energy production and molecule synthesis.

There is evidence that the apicoplast works in fatty acid and heme synthesis, like the leucoplast or in the production of ubiquinones that are important for the electron transfer chain in the mitochondria. There is also evidence that it is involved in FeS cluster production, like the hydrogenosome and mitosome. Both of these pieces of evidence show the interelationships of the endosymbiosed organelles and the connection between energy production and energy use. Whatever their functions are, if you destroy or inhibit it the malaria bug dies. As such, it has been a popular target for anti-malarial drugs.

Malaria parasites cured of their apicoplasts (cured means freed of) do not die right away. They just can’t invade any new cells and therefore can’t complete their life cycle. This is why anti-apicoplast drugs may be a boon to malaria treatment. The biosynthetic pathways in the apicoplast are the targets of four recent drugs, but the primary way to stop malaria remains the mosquito net. There is strong hope that a new vaccine, called RTS,S is a light at the end of the tunnel for this killer of millions.
The melanosome and the plastid have more in common.
The very rudimentary eye of some dinoflagellates
(dinos = rotating, and flagellum = whip) has a melanin-like
molecule in the pigment cup and the structure is called a
melanosome. However, it is of plastid orgin. The picture
above is of Polykrikos herdmanae. It has 8 transverse flagella,
as well as the pigmented eyespot to detect light sources.


One final thought on the plastid – an addition to the exception of melanosomes. We discussed a few weeks ago that melanosomes were the only organelles that could move from cell to cell. Well, that isn’t exactly so. I held off on adding the plastid to that list until we had discussed what a plastid was.

A 2012 study at Rutgers University tested whether plastids and mitochondria could move between plant cells. There results showed that entire plastid genomes could be seen in recipient cells, and the fact that the whole chromosome passed indicated that the plastid was probably moving from cell to cell intact. But there was no movement of the mitochondria, so it is a plastid (and melanosome) specific event.  The researchers hypothesize that this may be a way for plant cells to repopulate damaged cells with working organelles. As such, it would be similar to how mammalian stem cells can move mitochondria into damaged cells during tissue repair. But that is another story.

We have repeatedly talked about how the mitochondrion and plastid can replicate on their own and then are portioned out to the daughter cells when a parent divides. Can it really be that simple? I’ll bet there is a definite mechanism, and I bet that mechanism has exceptions. Let’s look into this next time.

Gregory Thyssena,Zora Svaba, and Pal Maligaa (2012). Cell-to-cell movement of plastids in plants Proc Natl Acad Sci U S A. , 109 (7) DOI: 10.1073/pnas.1114297109

For more information or classroom activties on plastids, gravitropism, or Plasmodium falciparum see:

Plastids –

Gravitropism –
207.62.235.67/case/biol215/docs/roots_gravity.pdf

Plasmodium falciparum –

Thursday, December 21, 2017

The Life Of The Party

Biology concepts – plant adaptations, osmosis, parthenogenesis

Last week we discussed the biological implications of an old Christmas carol. Today’s post is a hodgepodge of holiday biology, but we can still find some exceptions.


From a distance, spruce, fir, and pine Christmas
trees look similar. The differences are mostly in
the needles, both shape and number.
Christmas trees – There are many different types of trees used for Christmas, but they are all evergreens. This is the reason they were used in the first place. The tradition sprung from old pagan ceremonies that reminded us that spring would come and there would be a rebirth of greenery.

Evergreens have a thick wax coating on their needles (these are actually their leaves). This adaptation, as well as the low surface area of each leaf, helps to reduce water loss during the arid winter.

The resin of evergreens is higher in sugar than in other trees species. This keeps the liquids in the tree from freezing solid during the cold months. The higher sugar content oozes from the bark and at the collars of the branches, and is very sticky (picture Chevy Chase in Christmas Vacation).

Evergreen is a characteristic not a botanical grouping. They tend to photosynthesize all winter long, given enough water and sunlight. In deciduous trees there are hormonal (phytohormonal) signals that induce cleavage of the leaves from the stems (abscission) when there is not enough sunlight to justify making chlorophyll. In evergreens, there is some of this signal present, and pines do lose leaves in the winter, just not all of them. When cut and kept indoors, the abscission signal is increased, and together with the reduced water – all the needles end up on your carpet.


The leaves of cedar Christmas trees
look different from other evergreens.
If you choose a red cedar, just remember
that there is actually no evidence that
they keep moths away.
The groups of trees used for Christmas are members of the conifers – cedar, fir, and pine, and spruce. In general, pines have two or three needles coming from the same place on the twig, while fir and spruce usually have just one. To tell fir from a spruce, try to roll a needle in your fingers; if flat and won’t roll, it is probably a fir, but if it is four sided and can be rolled, it is a spruce. Cedars look different from the other three, they have scale-like leaves and ball cones, and their bark is more splintered.

Christmas cactus – This is a small genus of plants, comprised of two groups, the truncata and the buckleyi. In the wild, they grow on other plants (epiphytic) or on rocks (epilithic). They don’t have leaves, common in cacti, their flattened green stems serve as their photosynthetic elements. They occur in naturally in eastern Brazil, along the coast of the Atlantic Ocean. Those for sale in the U.S. are cultivars, bred for hardiness and different colors, different plants will bloom in red, yellow orange, or pink.


Thanksgiving cactus stem is shown on the
top, while the bottom stem is from a
Christmas cactus.
In Brazil, the cacti are called May Flowers, reflecting the month in which they bloom in the Southern Hemisphere. In the northern latitudes, they flower from November through January, depending on the cultivar. This presented a classic opportunity for commercialization.

You might want to look at your Christmas cactus a little more closely; you might actually have a truncata when you think you have a buckleyi. The Christmas cactus has stem segments that are rounded, with more symmetric points. The flowers hang down low and their pollen is pink. These flowers generally bloom later and these buckleyi cultivars therefore termed the Christmas cactus.


The yellow pollen on the left is characteristic of a Thanksgiving
cactus. The pink pollen of the flower on the right is typical of
the Christmas cactus.
In contrast, truncata cacti have much sharper stem segments. If it hurts to prune your cactus, you may have one of these. The flowers stay closer to horizontal, or even rise up on the plant. The pollen grains are yellow, so there are several ways to tell these plants apart. Perhaps the best way is by the blooming time. The truncata will bloom closer to the end of November. For this reason, they are often called Thanksgiving cacti. Still think you have a Christmas cactus?

Fruitcake – I am an unapologetic fruitcake fanatic. To everyone who isn’t - stop making fun and just send them to me.


Fruitcake! It may be my favorite
holiday treat.
The biology of fruitcake is based on bacteria, or more correctly, the lack of bacteria. The candied fruits used in fruitcake are not just dried, they are preserved. For many centuries, fruits were precious commodities, especially in the winter. The vitamin C and other nutrients were needed for good health, but spoilage kept most people from having them during the colder weather.

Meats were preserved with salt, called curing, since the days of the ancients. Fruits, on the other hand, don’t taste so good when salt cured. It turned out sugar that could preserve fruits just as salt cured meats. Either liquid syrup or crystalline sugar would do the job, but sugar was very costly. Honey could do the job, but not as well, and it wasn’t much more available. Therefore, preserved fruits were a luxury for some period of time.

With the advent of sugar beet production in the Americas in the late 1500’s and the resulting availability of sugar in Europe, there was a candied fruit glut in Europe. It became more common to use them in baking. Italian pannatone, and fruitcakes were common uses.

So how do salt and sugar preserve foods? It all has to do with water. Bacteria need water to survive; if you remove the water, you stop (or at least slow) bacterial growth. An osmotic gradient is set up when cells are placed in high salt (hypertonic) or high sugar environment. If the salt or sugar content is higher outside the cell, it means that the water concentration is higher inside the cell.


In osmosis, water flows from where there
is little solute toward where there is
much solute. In hypertonic solution,
this means water leaves the cell.
Water will flow from areas of high concentration to areas of low concentration, just as the salts and sugars will. This is diffusion, but in the case of water it is called osmosis (Plants That Don't Sleep Well). The solvent (water) and solutes (those things dissolved in the solvent) try to balance their concentrations, so water flows out of the cell and salts or sugars flow in. The result is pandemonium, chemical reactions are not possible under these conditions, and the organism either dies or goes into stasis.

Dehydration by salt and sugar work in several ways. One, removing water through osmotic pressure will turn the bacteria, fungi, and parasites already on the food to dried up corpses by pulling out their water. Second, the lack of water in the preserved food stops bacteria and other microbes that might land on them from propagating; no water, no cell division.

Third, the high salt or sugar concentrations, even with some water present, limits the species of organisms that could grow there. Only a few microbes, called halophiles (hal = salt, and phile = lover) can grow in high salt environments. Similarly, honey is only about 30% water, so not many bacteria can grow in this low water/high sugar environment (but some important bacteria can, so don't give raw honey to infants). Finally, the loss of water in the foodstuffs reduces the oxidation reactions that might take place to age the food. Fats are especially susceptible to oxidation, they go rancid in not too long. The curing of meats slows this process, but is less a problem in fruits due to the low fat content.

Those fruitcakes deserve a little more credit, don’t they? And by the way, fruitcakes are not the doorstops everyone thinks they are, they actually float in water.

Virgin birth – I will only touch on this subject, as the blog will soon be delving into a series of stories on mating and reproduction. There are many species of animal that can give birth to viable young without mating. This is called parthenogenesis (partheno = virgin, and genesis = birth).


In 2005, a komodo dragon in a zoo laid some
eggs. No big deal, except she hadn’t been housed
with a male for 2 years! Apparently, they can
reproduce sexually, or by parthenogenesis if
no males around. This has changed how
komodos are housed in zoos.
Parthenogenesis occurs when the unfertilized egg receives the messages necessary to begin to divide and form an embryo. The offspring have only their mother’s DNA with which to work, so they are all clones and all female. The egg does have two copies of the chromosomes, but this can occur in two ways. If the egg is haploid but undergoes chromosome doubling, the resultant offspring is a half-clone of the mother. But if the egg is produced only by mitosis, with no meiotic event to result in a haploid gamete, then the offspring is a full clone.

Many species use parthenogenesis exclusively, or in response to environmental or population conditions. Whiptail lizards, as well as aphids and some plants, are famous for undergoing parthenogenesis. No cases of mammalian parthenogenesis have been documented in the wild, but stem cells have been developed by parthenogenesis in the laboratory. Anyway, if the Christmas story was going to rely on parthenogenesis, then Jesus should have been a baby girl.


Mistletoe is an evergreen that grows
on other plants. It can draw water
from the host even in winter. It also
draws animals to the tree in winter.
Mistletoe – These are evergreen, hemi-parasitic plants that grow in many parts of the world. They have photosynthetic leaves, so they produce their own carbohydrates and energy, but they rely exclusively on their host tree for water and minerals. The mistletoe roots bore into the host bark and vascular tissue to obtain the water and minerals it needs.

The mistletoe can serve to hurt the host plant, especially if it grows too well, but they can also help the host. Junipers that harbor mistletoes produce more berries than those without. This is due to the large number of birds that come to eat the mistletoe berries; the juniper takes advantage. This makes it hard to determine of the symbiosis of mistletoe/host is parasitism or perhaps mutualism.


As the berry passes through the bird,
it releases sticky cellulose fibers that
help the seed stick to an unfortunately
placed branch.
The name, mistletoe, is not something commonly brought up at a holiday party. From the Old English word, “mistiltan,” the name tells it all. Birds eat the fruit and seeds of the plant and some of them pass through the GI tract unaltered. When excreted (mistil means dung), the sticky seeds may germinate on a limb (tan means branch). Interesting, but try not to mention it over a bowl of holiday punch.

The white berries of the mistletoe played a role in the 18th century Christmas kissing tradition. In Scandinavia, the maid under the mistletoe could be kissed, but the gentleman had to pull off a berry each time. While the berries were gone, the kissing privilege was lost. 

Next time we will finish our stories on sleep and activity by talking about introduced species. Then we will start a series of posts on the incredible worlds of water and salts in biology. Our fruitcake discussion above may serve as a great introduction, but it is just the tip of the iceberg.


The concepts discussed here will be discussed in more detail in other posts. Resources will be provided on those occasions.

Thursday, December 14, 2017

It’s A Plant World, We’re Just Living In It

Biology concepts – cell walls, chloroplasts, myco-heterotrophs, holoparasites,

Life on Earth is easy. It can be boiled down to three sentences. “The mitochondria and the chloroplasts are, in a fundamental sense, the most important things on Earth. Between them, they produce oxygen and arrange for its use. In effect, they run the place.” Lewis Thomas wrote this in his award winning book, The Lives Of The Cell: Notes Of A Biology Watcher, in 1975.


Nature’s carbon recycling center. The sun’s energy is used to 
polymerize carbon (CO2) into carbohydrates (CHO) and releases 
oxygen (O2). Then the mitochondria use the O2 to break down 
the CHO, resulting in chemical energy (ATP) and carbons (CO2) 
ready to be polymerized again.
He was so right - for the organisms that use them. I guess he didn't consider the exceptions. These two organelles mesh seamlessly in their functions. One produces carbohydrate and oxygen, while consuming carbon dioxide. The other consumes carbohydrate and oxygen and produces carbon dioxide. The ultimate recyclers.

If these two organelles are the most important things for life, then doesn’t that make plants the kings of life on Earth, since they have both chloroplasts and mitochondria? Makes you feel a bit more humble now about your place in world, doesn't it.

However, this brings up an essential question – and the main focus of today’s topic and exceptions. What makes a plant cell a plant cell? Green algae have chloroplasts and mitochondria, but they aren’t plants, they belong to the kingdom Protista. We have discussed the sea slug, E. chlorotica, and its ability to photosynthesize – it is certainly not a plant. So what makes a cell a plant cell?

Leaving the chloroplast out of the equation for a minute, you could argue that a plant cell is one with a cell wall and cell membrane. That surely separates them from animal cells, since animal cells only have the cell membrane. But many bacteria, archaea, fungi, and algae have cell walls. If the argument is refined to define a plant as having a certain kind of cell wall, then we must look a little closer. Many cell walls are made of sugars, but are plant cell walls unique in their constituents?


True bacteria have two large groupings, Gram+ and Gram -,
based on their cell wall structures. The gram stain sticks to
the peptidoglycan layer, so the thick layer on G+ bacteria make
them stain deeply. The lipopolysaccharide (LPS) layer of the G-
species keeps them from staining, and is highly toxic.
Endotoxin (LPS) and causes about 70% of septic shock cases.
Bacteria cell walls are made of peptioglycan (peptido = amino acid containing, and glycan = polymer of two sugars). One of the two components is always N-acetylmuramic acid, and the other is often poly-N-acetylglucosamine, but other things can be included as well. The exception is the Mycoplasma, a group of small bacteria that don’t have a cell wall at all. Since many antibiotics function by disabling the bacterial cell wall or preventing its formation, they don’t work against mycoplasma infections like M. genitalium, which a 2011 study linked to pelvic inflammatory disease in women.

Fungal cell walls are also made of a polysaccharide (poly = many, and saccharide = sugar), in a polymer called chitin. Chitin is also the rigid polymer that makes so many insects crunch when you step on them. Chitin cell walls are defining for fungi, as many cellulose containing cell wall fungi have been moved out of the kingdom of Fungi. But this still doesn’t tell us what is unique to plant cell walls.

Plant cell walls contain cellulose, and is complex. Plant cell walls can contain up to three layers, with different sugars involved, including cellulose, hemicellulose, and pectin, and lignin. Lignin is a more rigid polysaccharide that gives strength. It is what makes bark hard, protective, and water resistant.


If the hydrogens (H) bound to the #1 and #4 carbons
up on the same side, the polymer is starch. If they
are on different sides, the polymer is cellulose.
We can digest starch: we can’t digest cellulose.
Plants make both – the part we can’t digest we call
dietary fiber.
Cellulose is made of a chain of glucoses, yet we can’t digest it. The number one carbon in glucose has an –H that is sticking up or down. If the –H sticks “down”, then it is an alpha glucose. If it sticks “up”, then it is a beta-glucose. Cellulose is linked chains of beta-glucose. Starch is linked chains and branches of alpha-glucose. Just that difference in –H position determines if it is food for us or not. Herbivores have the enzymes (and bacteria) to digest cellulose, but not us.

So is it the inclusion of cellulose that makes a plant cell wall unique? Well, no. Algal cells also use cellulose in their cell walls. You might try to argue that algae are plants, since many of them also have chloroplasts and are primary producers – but you would be wrong. Algae can be unicellular (although they can also be multicellular) while plants are all multicellular. Algae don’t have specialized reproductive cells or parts like plants do; algae reproduce by spore or from broken parts of themselves. Finally, DNA analysis shows that while plants and algae are monophyletic (one ancestor), they diverged from one another long ago.

Then there is the issue that not every plant cell has a cell wall. In angiosperms (angio = chest or vessel, and sperm = seed; plants with enclosed seeds and flowers), the gamete (sex) cells of the male in the pollen and the gamete cells of the female in the ovary do not have cell walls, at least not on all sides. The ovary contains the ovules (latin for small egg), and the pollen contains the sperm cells and the tube cell, that forms the pollen tube and delivers the sperms cells to the ovules.

After the ovules are fertilized by the sperm cells of the pollen, the ovules form the seeds, and the ovary forms the fruit. From here on in, all the daughter cells will have cell walls. For fertilization, it would make sense that the involved cells would not have a cell wall that would just get in the way of love.


The Sago Palm isn’t a palm, but is one of the most
primitive plants that reproduces with seeds. It
presents a problem to pet owners because every part
is toxic to pets, but it tastes good to them. They don’t
know not to eat it; then they bleed to death.
And even weirder, not all plants use just this strategy. Cycads (like the sago palm, which isn’t really a palm at all), and gingko biloba plants have sperm cells with flagella, long projections that whip and move them along, hopefully toward an egg cell. They don’t use a tube cell or pollen tube; these plant cells without cell walls swim. Plant cells that move, now there is an exception worth noting! Some more primitive bryophyte plants (liverworts, mosses) also have motile sperm, but the cycads and gingko are the only examples of seed plants with motile cells.

So cell walls aren’t a defining characteristic of plant cells either. Maybe it is the chloroplast that defines a plant cell --- maybe not.

As you can guess, there are exceptions going both ways. There are organisms that have chloroplasts that aren’t plants, namely the algae. But a more interesting exception are many of the protozoan Euglenids. Euglena gracilis is a prototypical euglenid that can produce carbohydrate by photosynthesis. However, most euglenids can also eat things, which makes them both autotrophic and heterotrophic.

As for the other direction, there are many plants that don’t have chloroplasts. Of the roughly 350,000 different species of plants on earth, almost 3000 of them are non-photosynthetic. Therefore, the most common characteristic that people use to tell a plant from a non-plant (photosynthesis by chlorolplasts) isn’t true for almost 1% of the species on Earth. That is a pretty big exception. That would be like saying 1% of people on earth don’t have a brain! O.K., maybe that's a bad example.


Indian Pipe is Monotropa Uniflora. Monotropa means
one turn, and uniflora means one flower. The plant is
called the ghost plant – obvious, or the corpse plant –
because it turns black as it matures. This naming thing
is easy!
Indian pipe (Montropa uniflora, or ghost plant) is one such plant. Related to the blueberry of all things, the ghost plant has gone its own way and become parasitic. It garners its nutrients and energy from the tissue of another plant. The roots of the Indian pipe penetrate the rhizoids (root-like projections) of certain types of fungi and sponge off their hard work. In fact, the fungi themselves are symbiotic, having invaded the roots of certain pine tree species.

The fungus and tree live together in a mutualistic relationship, making the fungus a mycorrhizal (myco = fungus and rrhizal = root) variety. The tree supplies the fungus with carbohydrate, and fungus supplies the tree with mineral nutrients. However, Indian pipe does not respect this mutualism and is a parasite of the fungus, taking some of the carbohydrate supplied by the tree. This makes the Indian pipe a myco-heterotrophic parasite.

Other plants without chloroplasts are holoparasitic (gain nutrients only by parasitism).  These would include the rafflesia species of the Indonesian rainforests. These plants are know for having the largest single flowers in the world, some the size of car tires! The plant doesn’t have a stem or root or leaf, it is a vine that grows inside another type of vine. Only when it is ready to flower does it bud out from the bark of the host. The flower takes nine moths to develop, and then smells like rotting flesh in order to attract fly pollinators.


Rafflesia is also known as the corpse flower, as opposed
to the corpse plant (Indian pipe). This is because it
smells like a corpse in order to attract the flies that
pollinate it. This young man is either holding his breath,
has no sense of smell, or is just really odd.
In addition to holoparasitic plants, plant cells without chloroplasts would include those same gamete cells we discussed above as not having cell walls. And neither to do most root cells. However, there are exceptions, like many of the orchids. The ghost orchid has photosynthetic roots, which is a good idea, since they grow directly on other plants; their roots are not buried in the dirt.

Maybe it is not a single characteristic that makes a plant cell a plant cell, or a plant a plant. Maybe it is the combination of cells with cell walls, central vacuoles and in most cases, chloroplasts that make it a plant. I guess it is like beauty; you can’t define it, but you know it when you see it.

Next week we will take another shot at finding a defining characteristic of plant cells, namely the plastid, the mother of all chloroplasts – might there be an exception?


Mizukami I, & Gall J (1966). Centriole replication. II. Sperm formation in the fern, Marsilea, and the cycad, Zamia. The Journal of cell biology, 29 (1), 97-111 PMID: 5950730

Nikolov LA, Tomlinson PB, Manickam S, Endress PK, Kramer EM, & Davis CC (2014). Holoparasitic Rafflesiaceae possess the most reduced endophytes and yet give rise to the world's largest flowers. Annals of botany, 114 (2), 233-42 PMID: 24942001


For more information and classroom activities on cell walls or parasitic plants, see:

Cell walls –

Parasitic plants -
http://www.gardenbuildingsdirect.co.uk/Article/parasitic-plants